


Promiscuity Opens Paths for Coevolution
Evolution faces a challenge when physiological function depends on molecular partners recognizing one another like a precisely matched lock and key. If a mutation changes one partner, the interaction may be lost unless the other partner changes with it. But a coordinated change of two components is highly improbable. How, then, can a molecular recognition system evolve without harming its function along the way? In a study of plant reproduction, Amit Jangid of the Hebrew University of Jerusalem and his colleagues now propose a surprisingly biophysical explanation [1]. Their modeling shows how promiscuous interactions—molecular recognition that is not strictly one to one—allow an evolving molecular network to reorganize while retaining functionality. Applied to a long-standing puzzle of plant mating strategies, this promiscuity gives rise to a previously unknown type of coexistence of reproductive tactics [1].
Many flowering plants are hermaphrodites and have a choice whether to reproduce using their own pollen or using pollen from another plant. Each strategy has advantages. Self-fertilization guarantees reproduction when external pollen is scarce and transmits both parental copies of the genome to an offspring. Cross-fertilization, on the other hand, avoids the reduced fitness that often results from inbreeding. Classic evolutionary theory predicts that most populations tend toward one strategy or another [2]. However, empirical studies demonstrate that many plant populations use a mixture of both. For decades, biologists described the prevalence of mixed mating as an evolutionary enigma with unclear adaptive significance [3]. But proposed explanations—variable pollination conditions, patchy habitats, and other trade-offs—fail to address the molecular mechanism that underlies these mating strategies and how they evolve.
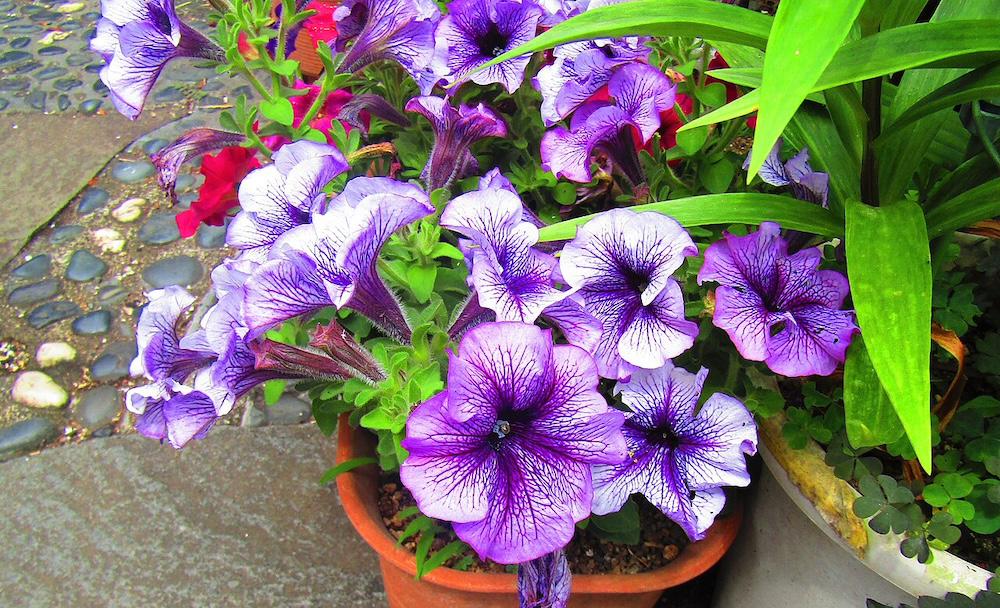
Plants commonly block self-fertilization with molecular recognition. In tomatoes, petunias (Fig. 1), apples, and their relatives, the female tissue produces a toxic enzyme called an RNase that harms pollen and stops fertilization. Pollen, meanwhile, carries a set of “antidote” proteins that can neutralize some RNases, allowing fertilization. Crucially, these antidotes can neutralize many different RNases but not the RNase associated with the pollen’s own mating type. Thus, pollen is rejected by plants of its own type but can fertilize plants of other types [4].
A population can therefore organize into distinct mating classes defined by molecular recognition types. If there are K equally represented classes, pollen is rejected by approximately 1/K of the population. Increasing the number of classes therefore reduces the reproductive cost of self-incompatibility [5]. But while classical population-genetic models have long recognized the importance of this number, they generally treat it as a prescribed parameter rather than explaining how the classes themselves arise and evolve.
To investigate the nature of mating classes, Jangid and colleagues model the interacting antidote and RNase proteins themselves. This is where the general problem of molecular recognition comes into play. The researchers treat each protein as a short string of amino acids. Two proteins bind only if the sum of their pairwise contact energies falls below a threshold. The threshold establishes how promiscuous binding is: More permissive binding allows a larger number of sequence “locks” to fit a given partner “key.”
This seemingly modest biophysical rule change transforms the evolutionary problem dramatically. The team’s previous work showed that promiscuity caused the population to self-organize into groups of mutually incompatible plants. New mating classes were born, while others died out [6]. The number of mating classes is thus an emergent property of the model rather than specified a priori and was found to be strongly affected by the antidote-RNase binding threshold.
The new work evaluates the plant population’s long-time reproductive strategy balance in terms of both the binding threshold and the fitness penalty associated with inbreeding. When self-fertilized seeds survive and thrive, the population becomes entirely self-fertilizing, and no mating classes form. When most self-fertilized seeds die and binding is sufficiently promiscuous, the population rejects self-pollen entirely and separates into mating classes. Between these extremes lies a third phase in which self-fertilizing and self-rejecting individuals coexist.
Earlier models also found coexistence but only in fixed proportions. Jangid and colleagues now find a new “volatile but persistent” state in which compatibility classes appear and disappear. The fraction of self-incompatible individuals changes substantially over time, yet the population does not collapse into either pure state. Importantly, no external noise drives these fluctuations.
Molecular promiscuity in recognition opens evolutionary pathways to resolve the coevolution conundrum. With promiscuous binding, many different molecular sequences bind equally well. As a result, function-preserving solutions form connected networks that evolution can traverse one mutation at a time. Laboratory experiments on bacterial protein pairs found such promiscuity as intermediate steps in evolution [7], and promiscuous regulatory interactions were shown to speed up the evolution of gene regulatory networks [8]. Jangid’s new study demonstrates that in addition to opening paths and speeding evolution, promiscuous molecular interactions can give rise to new dynamic states at the population level. Empirically testing the predicted volatile but persistent state and generalizing it to other molecular recognition systems remain open questions for future research.
References
- A. Jangid et al., “Volatile but persistent coexistence of self-compatibility and self-incompatibility in plants,” PRX Life 4, 043005 (2026).
- R. Lande and D. W. Schemske, “The evolution of self-fertilization and inbreeding depression in plants. I. Genetic models,” Evolution 39, 24 (1985); D. W. Schemske and R. Lande, “The evolution of self-fertilization and inbreeding depression in plants. II. Empirical observations,” 39, 41 (1985).
- C. Goodwillie et al., “The evolutionary enigma of mixed mating systems in plants: Occurrence, theoretical explanations, and empirical evidence,” Annu. Rev. Ecol. Evol. Syst. 36, 47 (2005).
- K. Kubo et al., “Collaborative non-self recognition system in S-RNase–based self-incompatibility,” Science 330, 796 (2010).
- D. Charlesworth and B. Charlesworth, “The evolution and breakdown of S-allele systems,” Heredity 43, 41 (1979).
- K. Erez et al., “The role of promiscuous molecular recognition in the evolution of RNase-based self-incompatibility in plants,” Nat. Commun. 15, 4864 (2024).
- C. D. Aakre et al., “Evolving new protein-protein interaction specificity through promiscuous intermediates,” Cell 163, 594 (2015).
- T. Friedlander et al., “Evolution of new regulatory functions on biophysically realistic fitness landscapes,” Nat. Commun. 8, 216 (2017).